
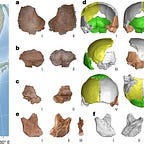
At position 996 of a collagen chain called COL1A2, the protein extracted from a right parietal bone from Xujiayao, a Middle Pleistocene site in the Nihewan Basin of northern China, carries lysine in 57 distinct peptides and arginine in one. The second Xujiayao specimen sampled, a mandibular ramus, gives 61 lysine-bearing peptides against a single arginine one. Every Denisovan with protein or genome data carries lysine at that position, while Neanderthals and modern humans carry arginine, and those two bones are the main reason the Xujiayao hominins are now being called Denisovan.
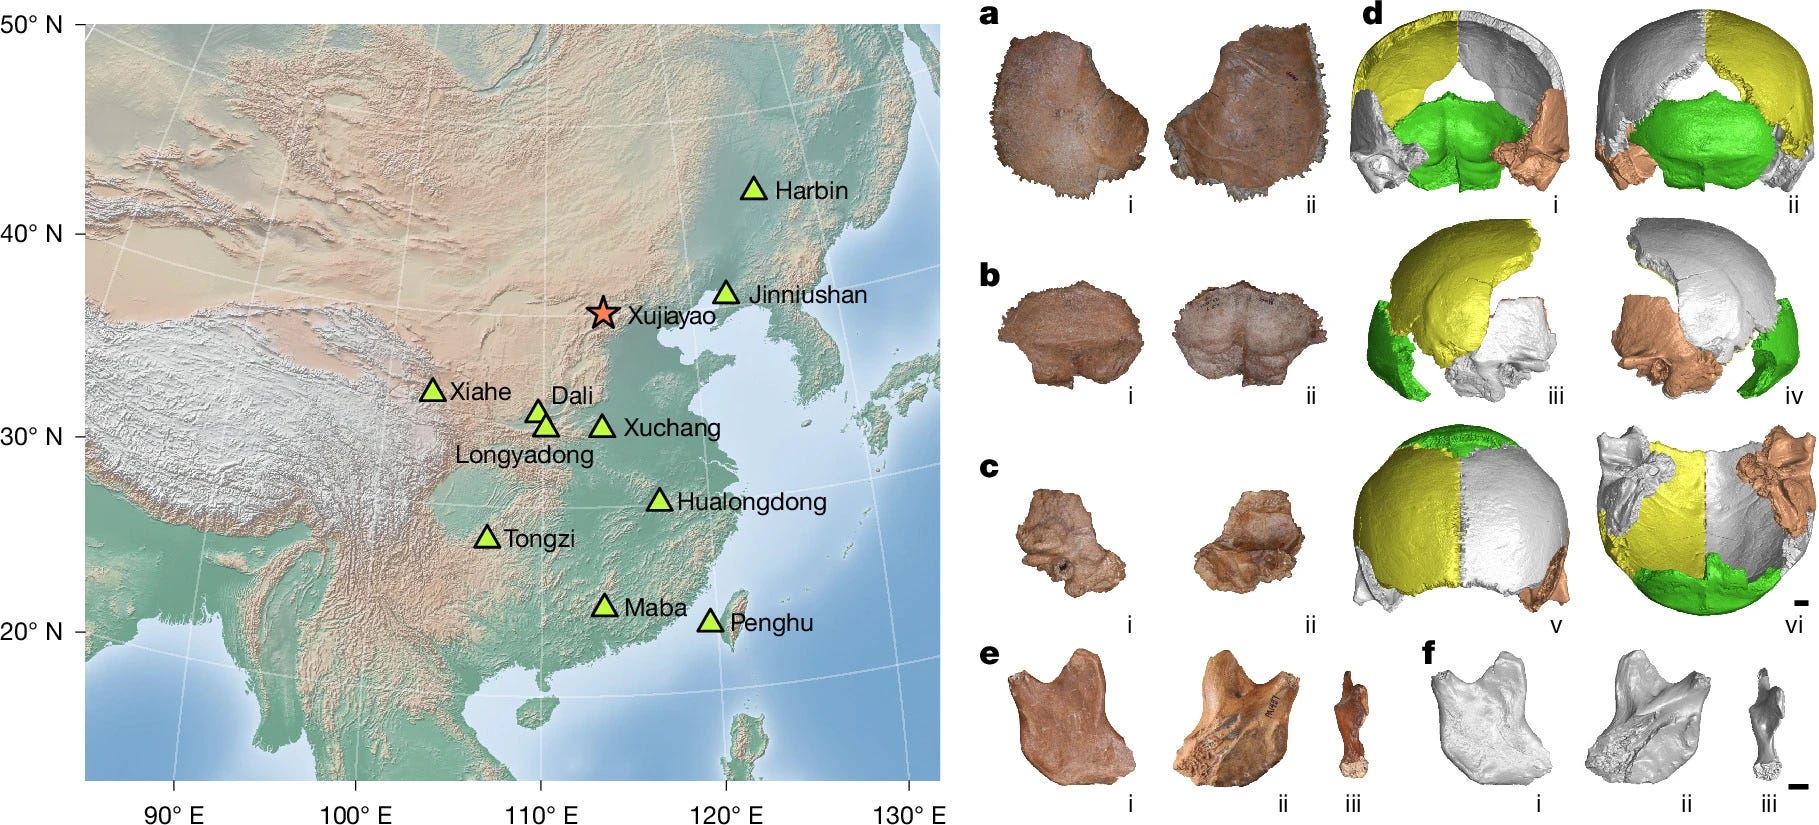
Since the fossils came out of the ground between 1976 and 1979, Xujiayao has been filed as Homo sapiens neanderthalensis, as early H. sapiens, as archaic H. sapiens, and, to avoid the argument, as archaic Homo. Most recently it became the holotype of Homo juluensis, a species proposed partly on the 1,700 ml endocranial capacity of the Xujiayao 6 cranium (Wu et al., Journal of Human Evolution, 2022)1. If you follow East Asian Middle Pleistocene hominins, you probably carry a picture of Dali, Jinniushan and Hualongdong as archaic humans with unsettled names, and of Denisovans as a lineage known from a genome plus a few molecularly confirmed jaws and one cranium.
The paper appeared in Nature2 on 21 October 2026. Song Xing, Zhongyou Wu, Qingfeng Shao and Junyi Ge are the equal-contribution first authors, and Qiaomei Fu of the Institute of Vertebrate Paleontology and Paleoanthropology in Beijing is the corresponding author. The team sampled two of the 20 Xujiayao cranial, mandibular and dental fossils, recovered 18 endogenous ancient proteins, and concluded that the assemblage belongs to a late Middle Pleistocene East Asian Denisovan population. They then compared skull and jaw anatomy across East Asian archaic Homo and argued that most of those fossils, Dali, Jinniushan and Hualongdong included, are Denisovan as well, and that the size gap behind H. juluensis is variation within one population. This post is about how much of that sweeping reclassification two bones and one amino acid can carry.
How do researchers know the proteins are ancient?
The sampling was minimal. The team CT-scanned both specimens first (37.56 μm resolution), then drilled a small hole in each in a dedicated clean room, shielding the surrounding bone with aluminium foil. They dissolved the powder, split the proteins into fractions, and digested them with trypsin, an enzyme that cuts proteins into short peptides. A mass spectrometer then reads the mass of each peptide fragment, which allows the amino acid sequence to be inferred. The runs were done in two independent laboratories, one at Capital Medical University and one at Fudan University, and the data were searched with two software packages, PEAKS Online and MaxQuant. Extraction blanks were processed alongside the samples, and a modern camel bone served as a positive control.
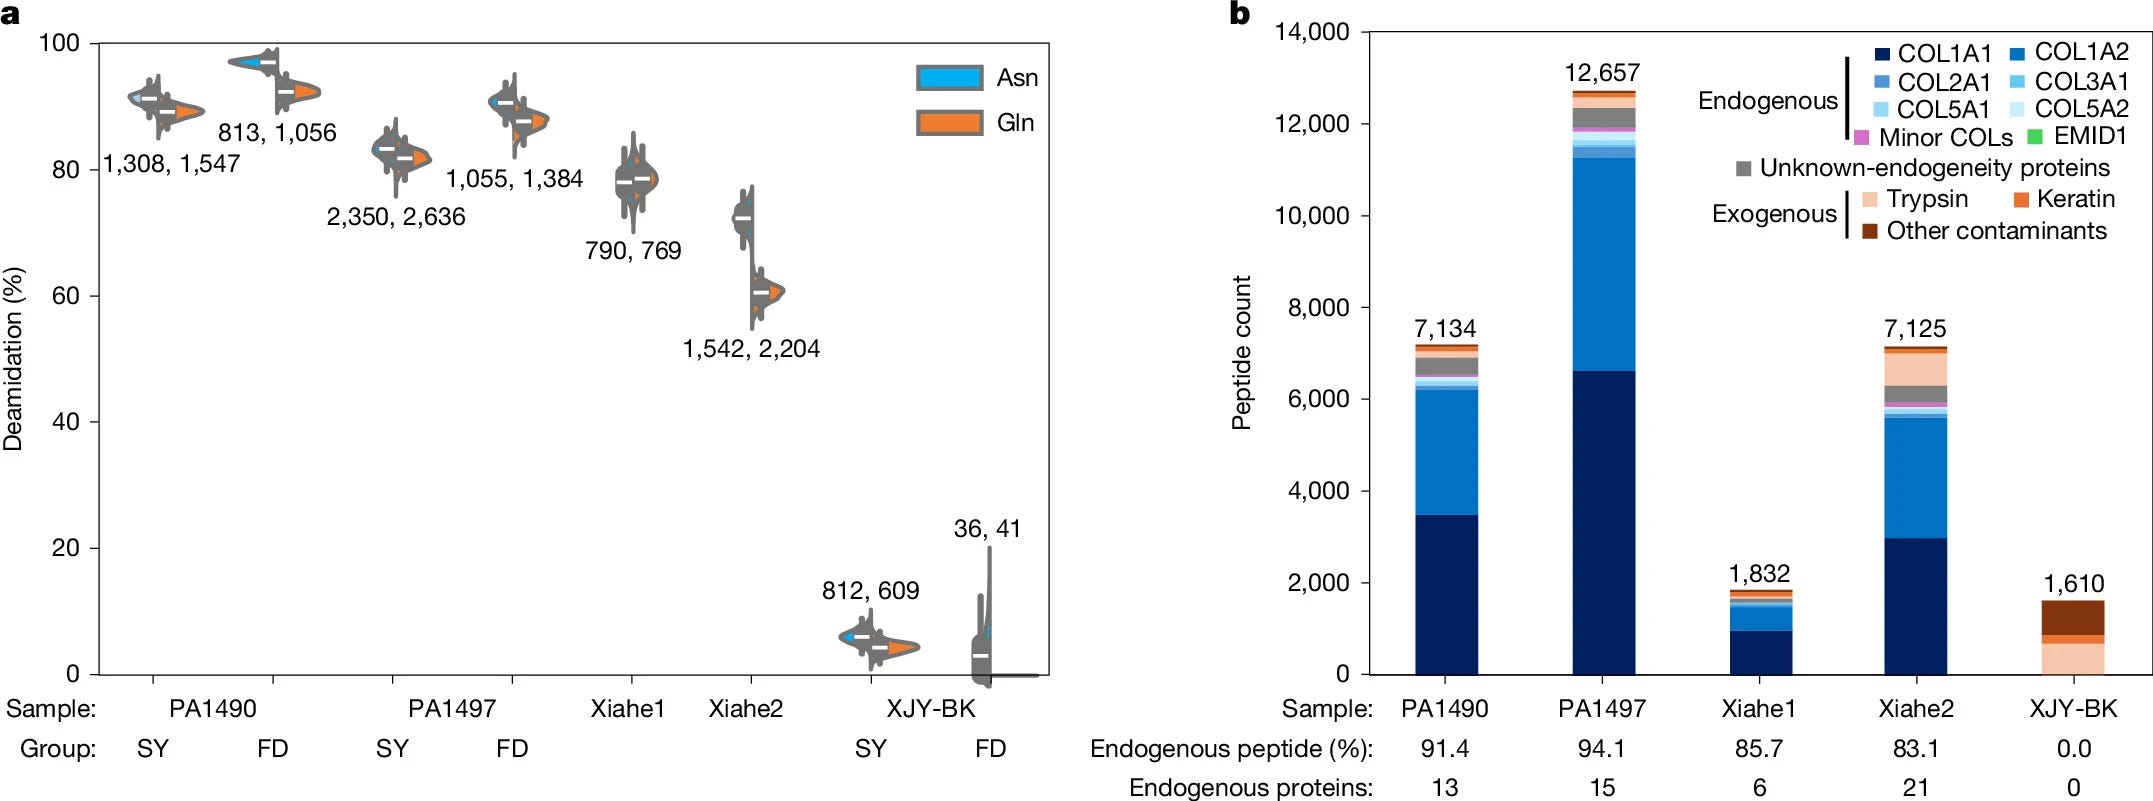
The hard part with any ancient protein is separating the real thing from modern contamination, and the authors lean on deamidation. Over long burial, the amino acids asparagine and glutamine slowly lose an amine group, so ancient proteins show high deamidation and fresh contaminants show little. In specimen PA1490 (the parietal), the main bone collagens had asparagine deamidation of 61.4 to 94.7% and glutamine deamidation of 44.9 to 92.6%, while keratins and trypsin, the usual contaminants, sat at 0.0 to 5.3% and 0.0 to 7.7%. PA1497 (the mandible) looks similar. After that filter, plus removal of peptides that could not be tied to a single gene, anything seen in the blanks, and anything MaxQuant could not confirm, 18 endogenous proteins remained: 13 for PA1490 and 15 for PA1497. Figure 2b gives the endogenous share of peptides as 91.4% for PA1490 and 94.1% for PA1497, and the extraction blank scores 0.0.
The taxonomic call comes in two steps. Searches against a mammalian type I collagen database placed both samples in the genus Homo, and the team then looked at single amino acid polymorphisms (SAPs), positions where sequences differ between lineages. The informative one is COL1A2-996. The paper’s Figure 3 shows the supporting peptides, 207 peptide-spectrum matches (individual spectra assigned to a peptide) for PA1490 and 244 for PA1497. The lysine peptides also show elevated deamidation at nearby residues (Asn977 at 69.2% and 69.4%, Gln1002 at 100% in both), which argues that they are genuinely ancient. The authors also built a Bayesian tree from 2,074 amino acid positions in eight proteins, with Denisova3, the Altai and Vindija 33.19 Neanderthals, 50 present-day humans from the Human Genome Diversity Project, and a chimpanzee (Pan troglodytes) as outgroup. Xujiayao and the Denisovans form a clade with posterior probability above 99%.
Within that clade the tree gives nothing: individuals fall into unstable arrangements with posterior probabilities below 50%, because no variant other than COL1A2-996K is shared. That is why the authors say only that Xujiayao is Denisovan in a general sense, without placing it relative to Xiahe, Penghu, Harbin or Denisova Cave. The dating, for what it is worth, is 199 to 138 ka from combined uranium-series and electron-spin-resonance methods (Shao et al., Quaternary Science Reviews, 2026)3, which makes Xujiayao about contemporary with the earliest confirmed Denisovans from northeastern China and southern Siberia.
Does skull shape make Dali and Jinniushan Denisovan too?
This is where I slow down, because the molecular result covers two bones and the morphological claim covers most of East Asia. With Xujiayao and Harbin both classed as Denisovan, the authors characterize a Denisovan skull. It has erectus-like traits (a low, wide neurocranium; a vault 7.7 mm thick at bregma and 12.0 mm at the parietal tubercle on Xujiayao 6), derived traits shared with later Homo (a strongly arched temporal squama), and a combination found in neither H. erectus nor modern humans: a low profile with near-parallel lateral walls, a nearly vertical but non-rounded occipital, and a mandible with a depression in the planum triangulare. They then check whether Dali, Jinniushan, Hualongdong and Xuchang show the same suite, and conclude that they do.
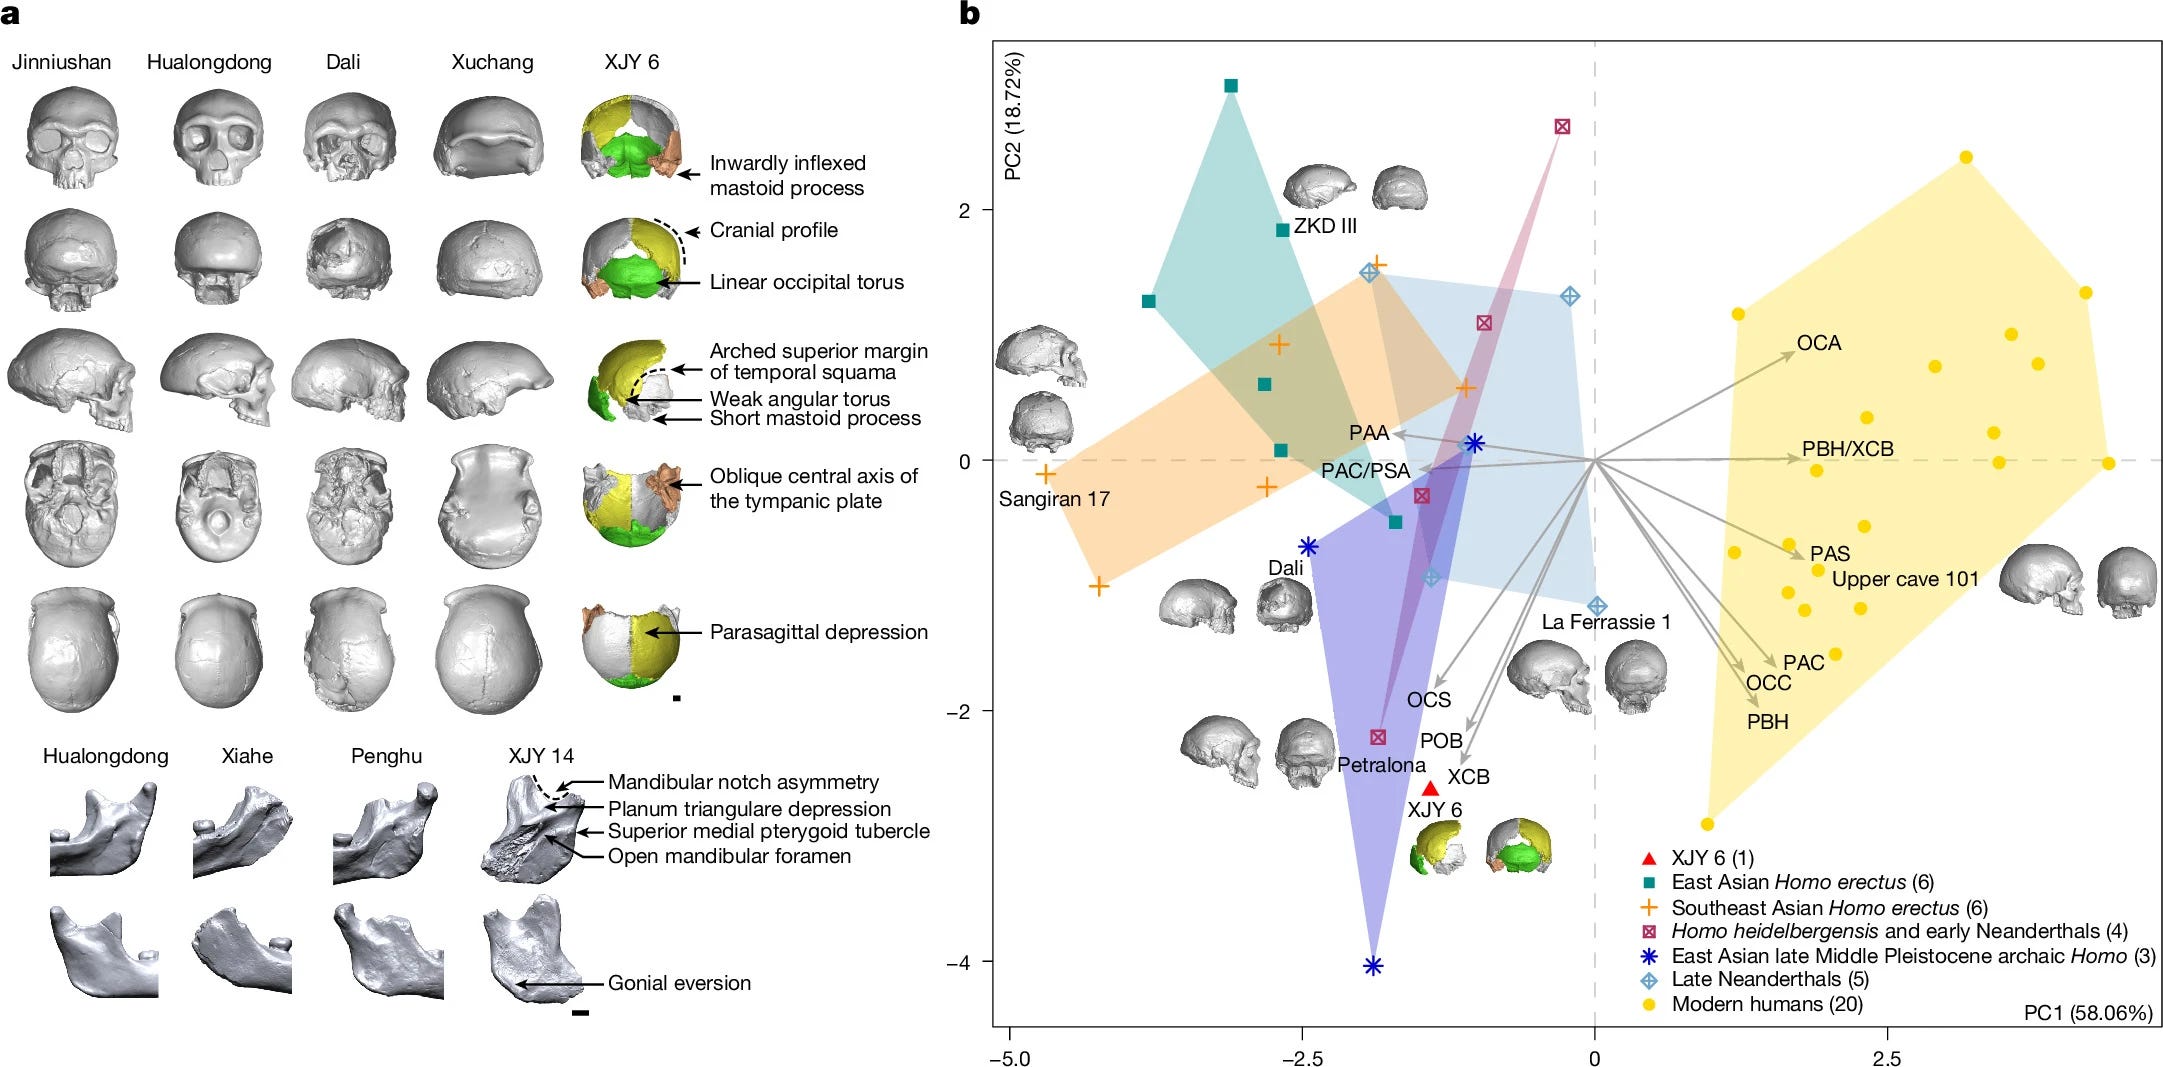
I find the Xujiayao assignment far stronger than that extension, for a reason the paper concedes itself: the suite “does not appear simultaneously in individual specimens but manifests in different forms or combinations across various specimens.” A definition that tolerates different combinations in different fossils is hard to falsify, and the definition was built from Xujiayao and Harbin before being tested on the rest. Hualongdong is the clearest case, since the paper says its mandibular features are only partly present, and it had previously been read as a transitional form toward H. sapiens. The principal component plot in Figure 4b has a comparison group of three East Asian late Middle Pleistocene archaic Homo specimens, against six East Asian H. erectus, six Southeast Asian H. erectus, four H. heidelbergensis and early Neanderthals, five late Neanderthals and 20 modern humans. Xujiayao 6 itself is a sample of one.
The H. juluensis argument deserves the same scrutiny. The authors point out that 1,700 to 1,800 ml for the Xujiayao and Xuchang group, against 1,120 to 1,420 ml for other East Asian late Middle Pleistocene Homo, falls inside the modern human range (1,090 to 1,880 ml) and the Neanderthal range (1,065 to 1,740 ml). That is true, but those ranges are species-wide, and the argument is that the gap is variation within one population. I would want the comparison made against variation within single populations, which the paper does not do. I also notice that the species proposal and the Denisovan assignment compete, and only the second now has molecular support.
What are the limits of the Xujiayao result?
The authors state several limits. The proteins cannot resolve relationships among Denisovans, and they add that incongruence between datasets might arise because the proteomic data are modest in amount. A test for a Penghu-specific variant (COL5A2-E1211V) returned no reliable evidence either way. Extra authenticity proxies were tried and not used because they were not examined with enough data. The Denisovan label for the other fossils rests on anatomy, and the paper offers the idea that admixture with early modern humans or other archaic groups reshaped late Neanderthal crania only as something that “might explain” the divergence.
Several weaknesses are not stressed. The assignment rests on a single variant, and the main text reports that no other variant is shared within the clade, so I could not tell how much of the >99% posterior depends on that one site. The consensus sequences also cover only eight proteins and 16.0% of the alignment. “Denisovan-specific” is itself defined by a small reference set: two Xiahe individuals, Penghu 1, Harbin and Denisova3 (Chen et al., Nature, 2019;4 Tsutaya et al., Science, 2025;5 Fu et al., Science, 20256), compared against Neanderthals and modern humans, so lysine at 996 has not been shown absent in every other Middle Pleistocene lineage. Two of 20 fossils were sampled, and the assemblage spans roughly 60,000 years of stratigraphy, so extending the result to every Xujiayao fossil assumes one population throughout. I could not find which layers the two sampled specimens came from. The paper reports no genome, and the dating gives no error ranges in the main text. The face of the Denisovan portrait comes from Harbin and other specimens, not from Xujiayao.
My verdict is that the Xujiayao result is convincing at the level the authors claim, a late Middle Pleistocene East Asian Denisovan population. Two bones, two laboratories, two search engines and a consistent deamidation signal make contamination an unlikely explanation for the lysine, and it fits the Xiahe, Penghu and Harbin picture. The wider reclassification of Dali, Jinniushan, Hualongdong and Xuchang is partly convincing at best, because it is a morphological argument built on a suite that no single fossil shows in full. Two things would settle it. One is more informative variants or DNA from additional Xujiayao individuals, ideally from different layers. The other is protein from the other fossils: the paper presents no molecular data for Dali, Jinniushan, Hualongdong or Xuchang, and if the Denisovan hypothesis is right, any of them that yields collagen should show lysine at COL1A2-996.
Wu, X.-J. et al. Evolution of cranial capacity revisited: a view from the late Middle Pleistocene cranium from Xujiayao, China. J. Hum. Evol. 163, 103119 (2022). https://doi.org/10.1016/j.jhevol.2021.103119
Xing, S., Wu, Z., Shao, Q., et al. The proteome of Middle Pleistocene Xujiayao and common Denisovan morphology. Nature (published online 21 October 2026). https://doi.org/10.1038/s41586-026-11132-z
Shao, Q. et al. New U-series and coupled ESR/U-series dating of Xujiayao (northern China), the type site for Homo juluensis. Quat. Sci. Rev. 373, 109742 (2026). https://doi.org/10.1016/j.quascirev.2025.109742
Chen, F. et al. A late Middle Pleistocene Denisovan mandible from the Tibetan Plateau. Nature 569, 409–412 (2019). https://doi.org/10.1038/s41586-019-1139-x
Tsutaya, T. et al. A male Denisovan mandible from Pleistocene Taiwan. Science 388, 176–180 (2025). https://doi.org/10.1126/science.ads3888
Fu, Q. et al. The proteome of the late Middle Pleistocene Harbin individual. Science 389, 704–707 (2025). https://doi.org/10.1126/science.adu9677


